
 Priscila Camelier1
 and Manoela Maria Ferreira Marinho2
PDF: Download Here | Cite this article
Associate Editor: Juan Mirande
Section Editor: Bruno Melo
Editor-in-chief: José Birindelli
Abstract
Uma nova espécie de Moenkhausia é descrita de um tributário do rio Teles Pires, bacia do alto rio Tapajós, Serra do Cachimbo, Estado do Pará, Brasil. A nova espécie é diagnosticada por um padrão de colorido distinto do corpo, que consiste em manchas escuras na porção anterior das escamas da segunda à sétima série longitudinal, uma mancha conspícua, alongada horizontalmente e em forma de gota no pedúnculo caudal, coloração única dos olhos em vida, com a porção dorsal da íris avermelhada e a porção ventral dourada brilhante, além de cinco ou seis raios ramificados na nadadeira pélvica. A nova espécie é morfologicamente semelhante a um grupo de congêneres amazônicos que compartilham o padrão de colorido incomum do corpo e olhos coloridos em vida, todas com distribuição restrita a áreas de planalto do escudo cristalino brasileiro. Este novo táxon representa a quinta espécie deste suposto grupo descrita da Serra do Cachimbo, cujos membros são provavelmente endêmicos da região, indicando que a Serra do Cachimbo pode representar uma importante região de endemismo para peixes de água doce de pequeno porte e ressaltando a necessidade de estudos taxonômicos e biogeográficos contínuos nas cabeceiras do escudo amazônico.
Palavras-chave: Amazônia, Endemismo, Padrão de colorido, Rio Teles Pires, Taxonomia.
Introduction
Moenkhausia Eigenmann, 1903 is among the three most species-rich genera within the Characiformes order (Dagosta, de Pinna, 2019; Marinho et al., 2021), with slightly more than 80 valid species that are widely distributed in the Neotropical Region, predominantly inhabiting the Amazon basin (Fricke et al., 2026). Molecular and morphological phylogenetic hypotheses of Acestrorhamphidae (whose members were until recently included in the former Characidae) have consistently indicated Moenkhausia as polyphyletic (e.g., Mirande, 2010, 2019; Oliveira et al., 2011; Mariguela et al., 2013; Ferreira et al., 2024), with less inclusive groups of species recovered as monophyletic. Although widely regarded as an artificial group, new species continue to be described under Eigenmann’s concept of Moenkhausia (e.g., Marinho et al., 2021; Marinho, Dagosta, 2023; Reia et al., 2024; Silva et al., 2025), which is the presence of the combination of two premaxillary teeth rows, the inner teeth row with five multicuspid teeth, complete lateral line, and caudal fin partially covered by small scales (Eigenmann, 1917).
Notably, Moenkhausia has a significant number of species recently described, with 24 (about 30% of its diversity) species described in the last decade, of which half were described with specimens collected in the “South American Characiformes Inventory” project (SACI). SACI (2011–2017) was a large-scale collaborative project focused on advancing the taxonomic and systematic knowledge of South American characiform fishes, integrating extensive field sampling in poorly collected regions with the sampled material deposited in major ichthyological collections, and combining morphological and molecular data to support taxonomic, phylogenetic, and biogeographic research. According to Marinho et al. (2019), the project brought together 34 participants from 17 institutions and conducted eight expeditions across Amazonian drainages (Brazil and Peru) and small coastal drainages of the Atlantic Forest, resulting in the processing of more than 31,000 specimens (3,500 lots) representing 972 species, with tissue samples obtained for many taxa. More than 60 new taxa have been described based on material collected by SACI, and several of these taxonomic outputs were compiled in a dedicated issue of Neotropical Ichthyology (see https://www.ni.bio.br/v12n2/).
During the latest expedition of this project, individuals of an undescribed species of Moenkhausia were collected in a tributary stream of the rio Teles Pires drainage that drains the Serra do Cachimbo, upper rio Tapajós basin, Amazon basin, Brazil. The new species described here represents one of the taxonomic outcomes resulting from this collaborative effort.
Material and methods
Morphometrics and meristics follow Fink, Weitzman (1974), except by the horizontal scale rows below the lateral line, counted to the pelvic-fin origin, and by posterior unbranched fin rays, which, besides the typical anteriormost unbranched rays, smaller unbranched rays that is eventually present posteriorly to the branched rays were counted separated from the later and are indicated as roman numerals (in the new species, they are present at the dorsal and pelvic fins), and with addition of distance from pelvic-fin origin to anal-fin origin. In the description, counts are followed by their absolute occurrence in parentheses. An asterisk indicates the count of the holotype. Standard length (SL) is expressed in millimeters (mm); other measurements are expressed as percentages of SL, except for subunits of the head, which are expressed as percentages of head length. Counts of supraneurals, branchiostegal rays, gill-rakers of first branchial arch, tooth cusps, small dentary teeth, unbranched anal-fin rays, procurrent caudal-fin rays, and position of pterygiophores were taken from cleared and stained (c&s) specimens prepared according to Taylor, Van Dyke (1985). Vertebrae of the Weberian apparatus were counted as four elements and the compound caudal centra (PU1+U1) as a single element. The pattern of circuli and radii was examined on scales sampled from the region between the lateral line and the origin of the dorsal fin. Color in life was taken on freshly collected material. Catalog numbers are followed by the number of specimens in alcohol and theSL range, and if any, the number of c&s specimens and their SL range or the presence of a tissue sample from specimens directly preserved in alcohol without fixation in formalin (mol). Institutional abbreviations follow Fricke, Eschmeyer (2026), with inclusion of the tissue collection of the Museu de Zoologia da Universidade de São Paulo (MZict).
Results
Moenkhausia nanah, new species
urn:lsid:zoobank.org:act:4387DA10-0633-430D-81CC-395F7569210B
(Figs. 1–4; Tab. 1)
Holotype. MZUSP 127625, 37.3 mm SL, Brazil, Pará State, Municipality of Novo Progresso, stream tributary of rio Inhandu, near to the locality “Olho da Xuxa”, rio Teles Pires basin, upper rio Tapajós basin, 09°29’12.5”S 55°08’12.9”W, 384 m above sea level, 17 Oct 2017, M. M. F. Marinho, O. T. Oyakawa, P. Camelier & R. Burger.

FIGURE 1 | Holotype of Moenkhausia nanah, MZUSP 127625, 37.3 mm SL, Brazil, Pará State, Novo Progresso, stream tributary of rio Inhandu, near to the locality “Olho da Xuxa”, rio Teles Pires basin, upper rio Tapajós basin.
FIGURE 2 | Paratype of Moenkhausia nanah, freshly preserved, MZUSP 124117, 33.6 mm SL, collected with the holotype.
Paratypes. INPA-ICT 62733, 5, 31.0–40.6 mm SL; MCP 56128, 5, 30.7–45.4 mm SL; MZUSP 124117, 106, 14.2–48.6 mm SL, 2 c&s, 34.1–36.2 mm SL, 2 mol (MZict 8885 and MZict 8886); ZUFMS 10126, 10, 26.5–40.3 mm SL, collected with the holotype.
Diagnosis. Moenkhausia nanah is distinguished from all congeners, except Moenkhausia cambacica Marinho, Ohara & Dagosta, 2021, M. chlorophthalma Sousa, Netto-Ferreira & Birindelli, 2010, M. parecis Ohara & Marinho, 2016, M. petymbuaba Lima & Birindelli,2006, M. plumbea Sousa, Netto-Ferreira & Birindelli, 2010, and M. solaris Silva, Santana & Marinho, 2025 by the presence of a dark blotch on scales of the second to seventh longitudinal series of body, which are formed by a higher concentration of chromatophores on the anterior portion of scales (vs. pigmentation absent or, when present, concentrated at the middle or posterior margin of scales, forming stripes or a reticulate pattern, as in M. sanctaefilomenae species group). The new species can be distinguished from all aforementioned species, except M. plumbea, by having five or six branched pelvic-fin rays (vs. seven).It can be distinguished from M. plumbea and, additionally, from M. chlorophthalma and M. petymbuaba, by the absence of a conspicuous longitudinal dark stripe on body (vs. dark stripe present). Additionally, Moenkhausia nanah is distinguished from all aforementioned species by having the upper portion of iris markedly red in life (vs. eyes crossed by a longitudinal dark stripe without red pigmentation in M. cambacica and M. plumbea, green in M. chlorophthalma,blue in M. parecis, mostly green with some red in M. petymbuaba, and dark in M. solaris).
Description. Morphometric data of the holotype and paratypes presented in Tab. 1. Largest examined specimen 48.6 mm SL. Body laterally compressed, moderately deep. Greatest body depth at vertical through tip of adpressed pectoral fin. Dorsal profile of head convex from upper lip to vertical through anterior nostrils, slightly convex from that point to the vertical through middle of eye, straight to slightly concave from latter point to tip of supraoccipital spine. Dorsal profile of body slightly convex from tip of supraoccipital spine to dorsal-fin origin, straight along dorsal-fin base, straight from that point to adipose-fin origin, and somewhat straight to slightly concave from adipose fin to origin of anteriormost dorsal procurrent caudal-fin ray. Ventral profile of head and body slightly convex from tip of lower jaw to anal-fin origin, straight along anal-fin base, and slightly concave from the terminus of anal fin to origin of anteriormost ventral procurrent caudal-fin ray.
Jaws vertically aligned, mouth terminal. Premaxillary teeth in two distinct rows (Fig. 3). Outer row with 3(6), 4*(20), or 5(3) tricuspid teeth. Inner row with 4(2) or 5*(27) teeth bearing three to five cusps. Posterior terminus of maxilla at the vertical through middle of pupil. Maxilla approximately at 45 degrees angle relative to longitudinal axis of body. Maxilla with 2*(20) or 3(9) teeth, with four or five cusps. Dentary with 4*(24) or 5(1) larger teeth decreasing in size posteriorly, with four or five cusps, followed by 6(2) diminute conical to tricuspid teeth. Central median cusp in all multicuspid teeth more developed than remaining lateral cusps. Branchiostegal rays 4(2). First gill arch with 2(2) gill rakers on hypobranchial, 8(2) rakers on ceratobranchial, 1(2) raker on intermediate cartilage, and 5(2) rakers on epibranchial. Infraorbitals 5(2), except in one specimen, which has 6 on the left side and 5 on the right, the latter side showing partial fusion of infraorbitals 4 and 5. Nostrils close to each other, anterior opening circular and small, crescent-shaped posterior one, twice in size. Nostrils separated by narrow skin flap.
TABLE 1 | Morphometric data of Moenkhausia nanah. Range includes the holotype. N = number of specimens; SD = Standard deviation.
| Holotype | N | Range | Mean | SD |
Standard length (mm) | 37.3 | 30 | 26.5–48.6 | 34.7 | – |
Percentage of standard length | |||||
Depth at dorsal-fin origin | 30.6 | 30 | 27.3–34.1 | 31.4 | 1.6 |
Snout to dorsal-fin origin | 56.6 | 30 | 54.4–58.7 | 56.3 | 1.1 |
Snout to pectoral-fin origin | 27.9 | 30 | 25.8–31.1 | 28.1 | 1.0 |
Snout to pelvic-fin origin | 48.8 | 30 | 47.7–52.9 | 50.0 | 1.2 |
Snout to anal-fin origin | 65.1 | 30 | 63.4–68.0 | 65.8 | 1.2 |
Caudal-peduncle depth | 11.5 | 30 | 10.3–12.9 | 11.5 | 0.6 |
Caudal-peduncle length | 11.0 | 30 | 8.5–13.2 | 11.3 | 1.0 |
Pectoral-fin length | 19.3 | 30 | 18.9–23.5 | 21.3 | 1.0 |
Pelvic-fin length | 13.7 | 30 | 13.3–16.9 | 14.9 | 1.0 |
Pelvic-fin origin to anal-fin origin | 17.4 | 30 | 15.7–18.8 | 17.3 | 0.7 |
Dorsal-fin base length | 12.9 | 30 | 11.6–14.7 | 13.1 | 0.8 |
Dorsal-fin length | 23.9 | 30 | 23.9–28.8 | 26.0 | 1.2 |
Anal-fin base length | 25.7 | 30 | 24.3–26.9 | 25.6 | 0.7 |
Anal-fin length | 17.7 | 30 | 15.4–21.5 | 18.2 | 1.3 |
Eye to dorsal-fin origin | 41.3 | 30 | 39.1–42.4 | 40.8 | 0.9 |
Dorsal-fin origin to caudal-fin base | 46.6 | 30 | 45.1–51.7 | 48.8 | 1.8 |
Head length | 32.4 | 30 | 27.4–32.4 | 30.0 | 1.1 |
Percentage of head length | |||||
Horizontal eye diameter | 29.8 | 30 | 27.8–35.2 | 31.4 | 2.2 |
Snout length | 25.6 | 30 | 24.1–29.6 | 25.9 | 1.4 |
Interorbital width | 30.6 | 30 | 26.9–34.4 | 30.6 | 1.8 |
Upper jaw length | 44.6 | 30 | 42.3–50.0 | 46.3 | 2.2 |
Scales cycloid, moderately large, with 10 to 17 parallel radii from focus to posterior border and several conspicuous circulii anteriorly. Lateral line slightly curved downward anteriorly, with 33(3), 34*(13), 35(10), or 36(4) perforated scales continuously from supracleithrum to caudal-fin base. Longitudinal scale rows between dorsal-fin origin and lateral line 5*(26) or 6(4). Longitudinal scale rows between lateral line and pelvic-fin origin 4(2) or 5*(28). Predorsal scales variably arranged. Some specimens with 11(1), 12(4), or 13(2) scales arranged in a median series. Others with anterior portion of predorsal region covered by scales from 1st*(14) or 2nd(8) longitudinal scale row, irregularly arranged, followed by single series of 10(8), 11*(11), or 12(3) median scales. Single row of 8(1), 9(3), 10(11), 11(4), or 12*(3) scales covering base of anteriormost anal-fin rays. Axillary scale absent. Horizontal scale rows around caudal peduncle 14(9), 15*(17), or 16(4). Caudal fin with small scales on the basal fourth of caudal-fin lobes.

FIGURE 3 | Jaws of Moenkhausia nanah, MZUSP 124117, 36.9 mm SL, paratype. Lateral view of upper jaw (A) and medial view of lower jaw (B).
Supraneurals 5(1) or 6(1), without bony lamella. Dorsal-fin rays ii*(30), 9*(27) or 8,i(3). Dorsal-fin origin posterior to vertical through pelvic-fin origin. First dorsal-fin pterygiophore located behind neural spine of 11th(2) vertebra. Base of last dorsal-fin ray slightly anterior to vertical through anal-fin origin or aligned with anal-fin origin. Adipose fin present. Anal-fin rays iv(2), 17(2), 18(13), 19*(14), or 20(1); anteriormost rays longer, subsequent rays gradually decreasing in size. Pectoral-fin rays i*(30), 10*(20) or 11(10). Pelvic-fin rays i*(30), 6*(23) or 5,i(7). Anteriormost anal-fin pterygiophore inserted posterior to haemal spine of 18th(2) vertebra. Principal caudal-fin rays i,8/9,i(1), i,9/7,i(1), i,9/8,i*(25), or i,9/10,i(1); caudal fin forked, lobes somewhat pointed, of similar size. Dorsal procurrent caudal-fin rays 10(2); ventral procurrent caudal-fin rays 9(2). Total vertebrae 35(2): precaudal vertebrae 17(2) and caudal vertebrae 18(2).
Coloration in alcohol. Overall ground coloration pale or yellowish, with small dark chromatophores spread at the entire head and body, densely concentrated in the dorsal portion (Fig. 2). Jaws, opercular, and infraorbital areas pigmented with dark chromatophores. A dark blotch on each scale of the second to seventh longitudinal body series formed by a higher concentration of chromatophores on the anterior portion of scales. Single, dark humeral blotch, vertically oriented, extending two or three scale rows above and one scale row below the lateral line. Middle portion of humeral blotch wider, over three scales horizontally. Ventral portion narrower, spanning over one scale. Some specimens with a vertical pigmented area posterior to the humeral spot. Thin longitudinal dark stripe at horizontal septum, formed by underlying chromatophores extending from vertical through dorsal-fin origin to caudal peduncle. A conspicuous dark horizontal drop-shaped blotch on the caudal peduncle, usually tapering anteriorly, extending to middle caudal-fin rays, never reaching the upper and lower edges of caudal peduncle. All fins with dark chromatophores scattered along edge of lepidotrichia. Some specimens with concentration of dark chromatophores on distal portions of dorsal and anal fin-rays.
Coloration in life. Dorsal portion of head and body darker than ventral portion. Ventral half of head and body golden yellow (Fig. 4). Middle portion of body greenish anteriorly and light pink posteriorly. Infraorbital and opercular areas reddish, more intense on opercular area. Some specimens retaining guanine on infraorbital, opercular, and gular areas. Edge of lips dark. Dorsal portion of eye red with a bluish-purple line between this part and the iris, ventral portion bright golden with light greenish hue. Humeral blotch inconspicuous in life. Black caudal-peduncle spot conspicuous. All fins with intense orange to yellow coloration. Anal fin and caudal-fin lobes orangish. Posterior tip of caudal, anal, and dorsal fins with concentration of dark chromatophores, more evident at caudal and anal fins. Distal portions of dorsal, anal, pelvic, and caudal fins hyaline.
Sexual dimorphism. No secondary sexually dimorphic characters were found among analyzed specimens.
Geographical distribution. Moenkhausia nanah is known only from its type locality, a stream tributary of rio Inhandu, near to the locality “Olho da Xuxa”, rio Teles Pires basin, upper rio Tapajós basin at Serra do Cachimbo, Novo Progresso, Pará State, Brazil (Fig. 5A).
Ecological notes. Moenkhausia nanah was collected in a dark water stream (Fig. 5B), running over rocks, organic debris, and sand bottoms, at an altitude of approximately 380 m above sea level, in a habitat characterized by moderate water current. Aquatic macrophytes were present in abundance and the riparian vegetation is mainly composed of herbs, shrubs, and trees. The analysis of stomach contents of two c&s specimens (MZUSP 124117, 34.1–36.2 mm SL) revealed the presence of allochthonous and autochthonous items, composed of filamentous algae, fragments of vascular plants, organic debris, nymph of Ephemeroptera, Simuliidae larva (Diptera) and fragments of other insects (Coleoptera and other unidentified orders).

FIGURE 4 | Moenkhausia nanah, live specimen, paratype, MZUSP 124117, 48.6 mm SL, Brazil, Pará State, Novo Progresso, rio Teles Pires basin, upper rio Tapajós basin.
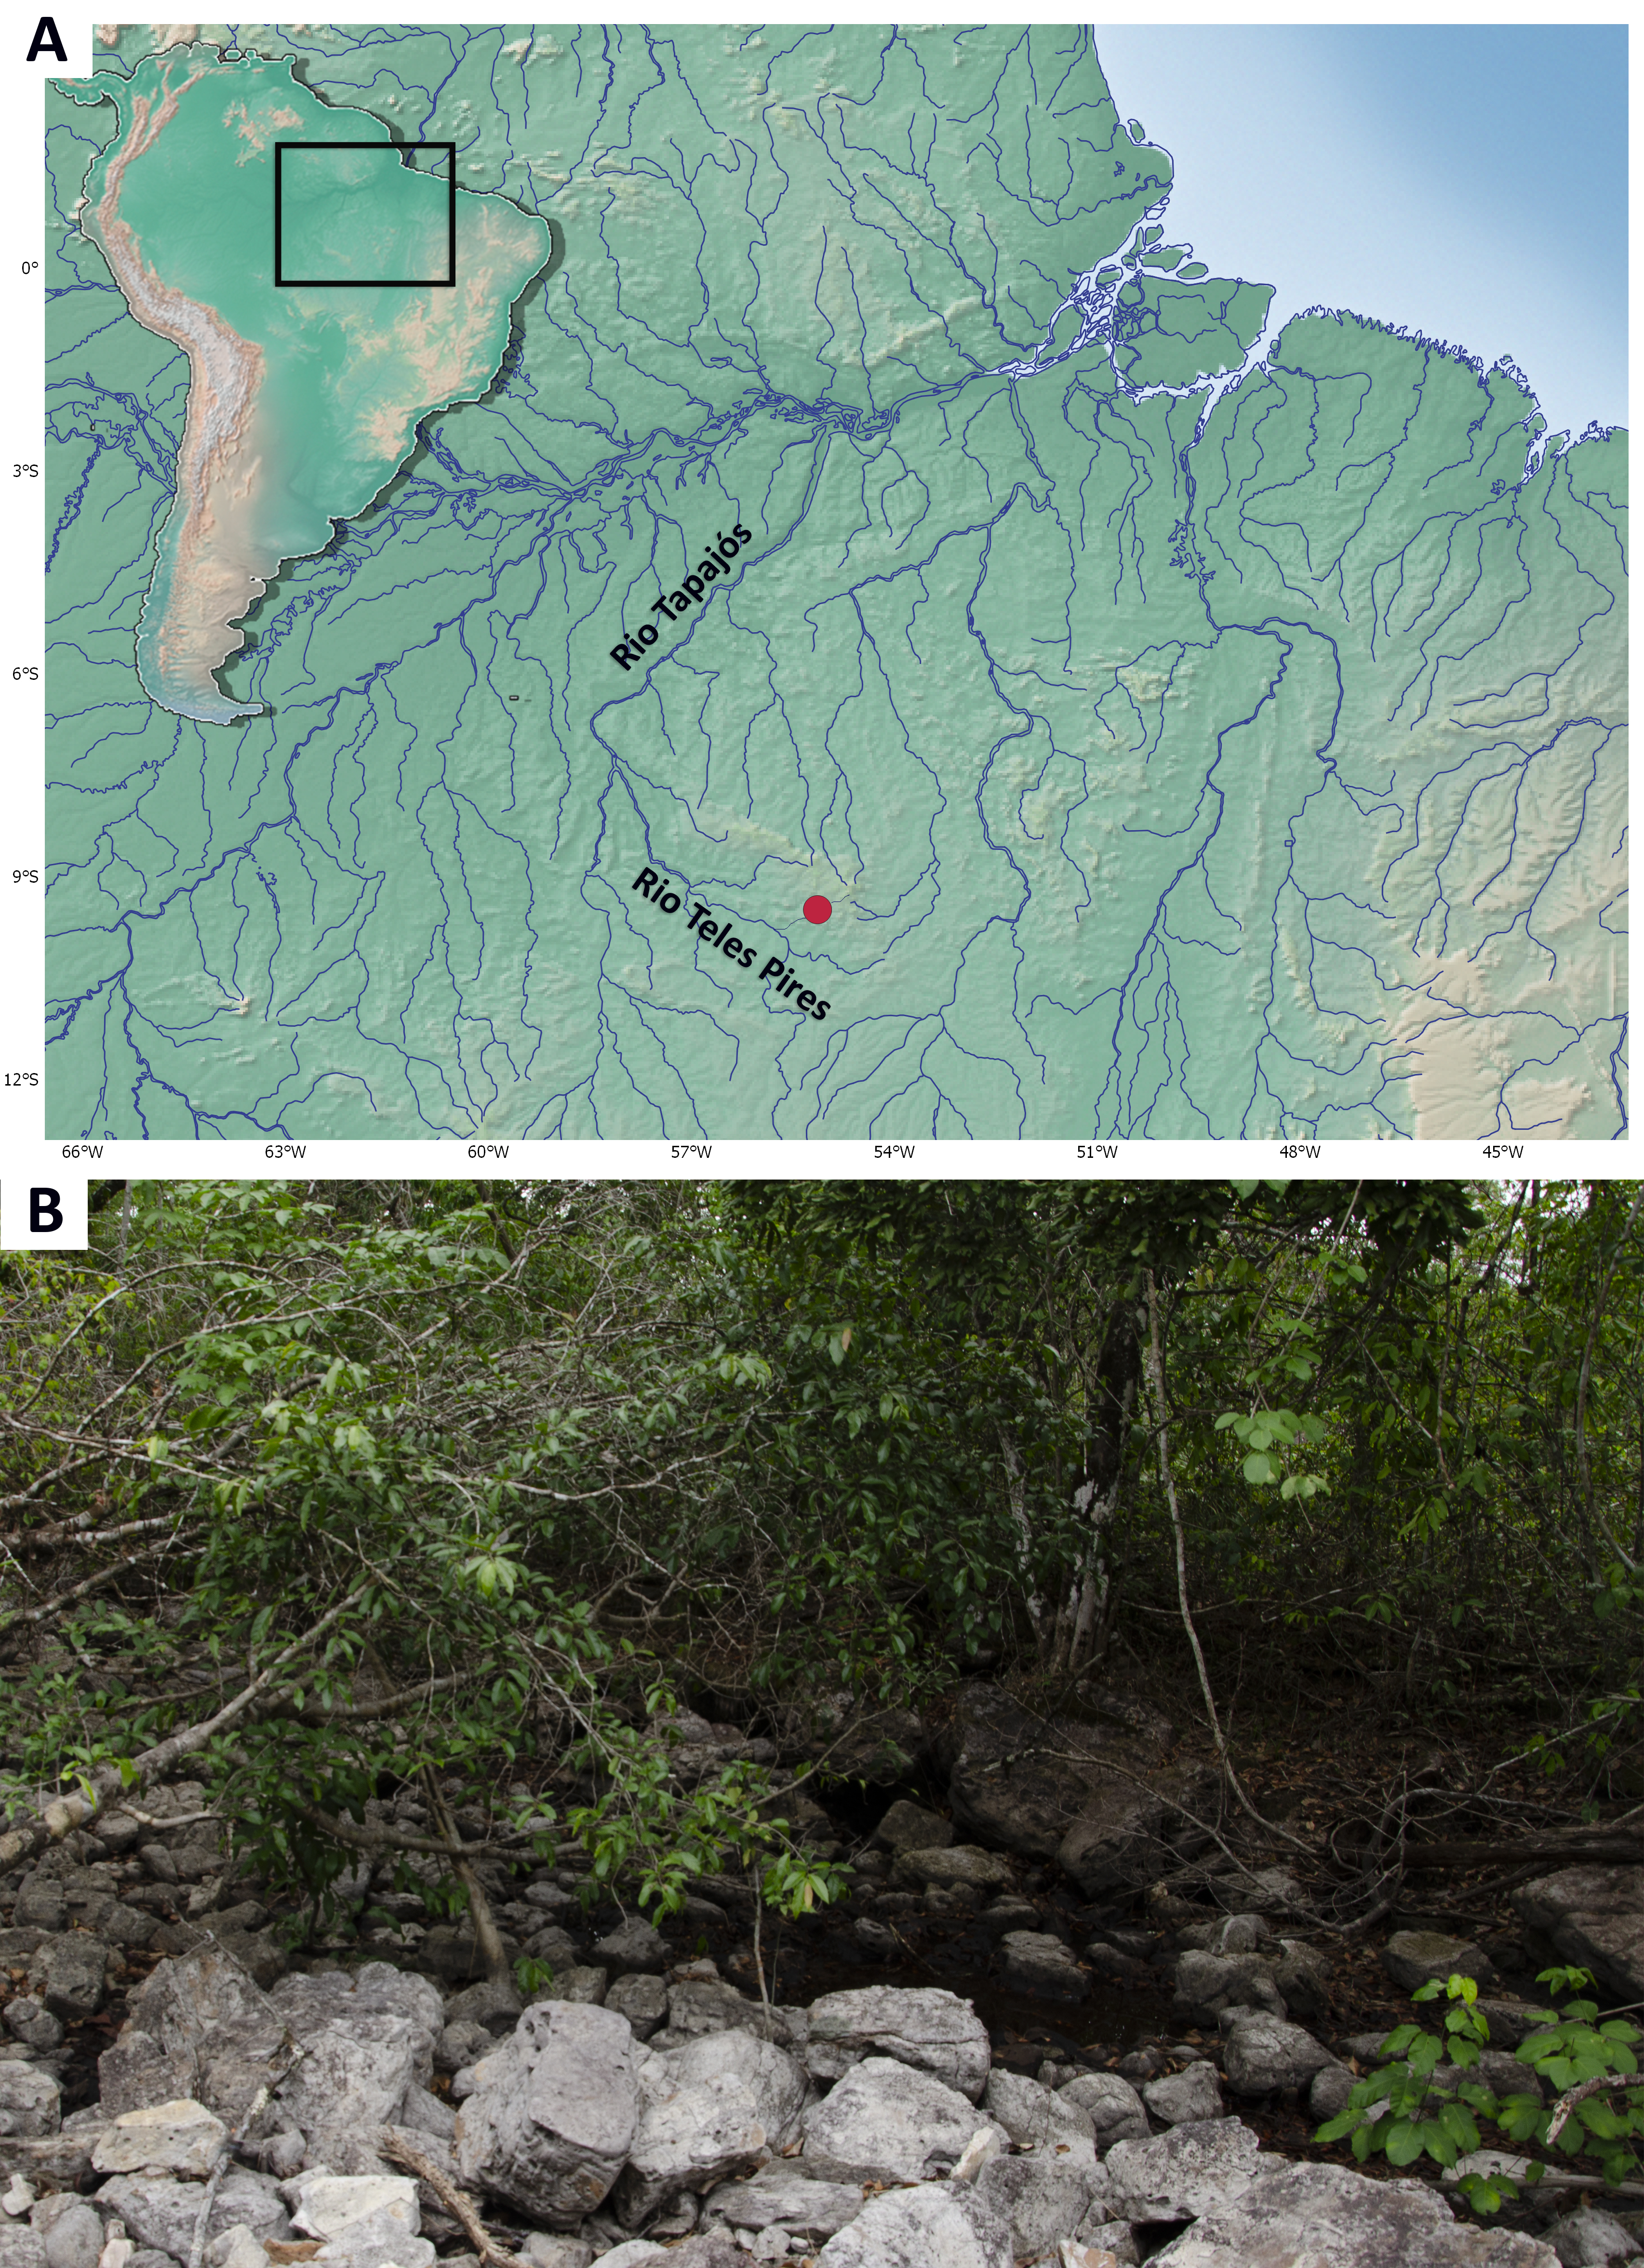
FIGURE 5 | Geographical distribution of Moenkhausia nanah (A) and its type-locality, a small stream tributary of the rio Inhandu, rio Teles Pires basin, upper rio Tapajós basin, Pará State, Brazil (B).
Conservation status. Moenkhausia nanah is currently only known from its type locality, a tributary of the rio Inhandu, upper rio Teles Pires basin, rio Tapajós basin, restricted to the Serra do Cachimbo region. Despite its restricted distribution, the area is well preserved, and no identifiable threats have been recorded. Therefore, Moenkhausia nanah should be classified as Least Concern (LC) following the International Union for Conservation of Nature (IUCN) categories and criteria (IUCN, 2024).
Etymology. The specific name, nanah, is in honour of the esteemed ichthyologist Dr. Naércio Aquino Menezes in recognition of his significant contributions to the knowledge of ichthyofauna. Naércio, who we affectionately call “Naná”, trained many new ichthyologists with respect and kindness and was our PhD advisor. Dr. Menezes also coordinated the “South American Characiformes Inventory” project, which supported the expedition in which the new species was collected. A noun in apposition.
Discussion
The phylogenetic relationships among species currently assigned to Moenkhausia remain poorly resolved. Phylogenetic studies have consistently recovered Moenkhausia as a polyphyletic group (e.g., Mirande, 2010, 2019; Mariguela et al., 2013), with important consequences for the delimitation and recent reclassification of the genus (see Melo et al., 2024; Silva et al., 2025). Those phylogenetic studies also have recovered less inclusive groups of species as monophyletic. Several of these clades had long been hypothesized as monophyletic based on the shared presence of distinctive color patterns. One example involves a group of species that, until recently, was allocated to Moenkhausia but has since been transferred to the genus Bario Myers, 1940 by Melo et al. (2024). This group, comprising Bario australis(Eigenmann, 1908), B. cosmops (Lima, Britski & Machado, 2007), B. forestii (Benine, Mariguela & Oliveira, 2009), B. oligolepis (Günther, 1864), and B. steindachneri (Eigenmann, 1893), was also recovered as monophyletic in previous phylogenetic studies (see Mariguela et al., 2013; Mirande, 2019; Ferreira et al., 2024) and recognized by several authors as closely related taxa (e.g., Costa, 1994; Lima, Toledo-Piza, 2001; Lima et al., 2007). These species share a reticulated color pattern of the body, a large dark blotch at the caudal peduncle and caudal-fin basis with a clear area preceding it, and a red pigmentation on the dorsal portion of the eye.
An additional putative monophyletic group, never tested within a phylogenetic framework, includes Moenkhausia cambacica, M. chlorophthalma, M. parecis, M. petymbuaba, M. plumbea, M. solaris,and the new species herein described. All of them exhibit a unique color pattern consisting of a series of dark blotches on body, located at the anterior portion of scales, not observed in any other species of the family (see Sousa et al., 2010; Marinho et al., 2021; Silva et al., 2025). Additionally, these species possess distinctive eye coloration, such as entirely green in M. chlorophthalma, partially green in M. petymbuaba, totally blue in M. parecis, yellowish with a longitudinal dark stripe in M. plumbea and M. cambacica (Marinho et al., 2021; Silva et al., 2025), and red in M. nanah. These authors suggest that these species are likely closely related, although further phylogenetic analyses are required to confirm this hypothesis.
The currently known geographic distribution of Moenkhausia nanah is highly restricted, encompassing an upper tributary of the rio Teles Pires within the Serra do Cachimbo. The other putative closely related species, M. cambacica, M. chlorophthalma, M. petymbuaba, M. plumbea, M. parecis, and M. solaris, also exhibit narrow distributions, being endemic to elevated areas of the Brazilian Shield. Moenkhausia chlorophthalma, M. nanah, M. petymbuaba, M. plumbea, and M. solaris are confined to headwaters of the Xingu and/or Tapajós basins draining the Serra do Cachimbo whereas M. cambacica and M. parecis are restricted to the upper rio Madeira basin at the Chapada dos Parecis. This pattern indicates a recurrent endemism within the putative group, associated with upland regions of the Brazilian Shield, particularly the Serra do Cachimbo, and the Chapada dos Parecis, likely driven by the pronounced topographic heterogeneity of the region, promoting both long-term isolation and faunal interchange among headwaters. The biogeographic analysis conducted by Dagosta, de Pinna (2017) provides further support for this interpretation, recovering the rio Iriri (rio Xingu basin) as closely related to the rivers Jamanxim, Juruena, and Teles Pires (rio Tapajós basin), thus defining a biogeographic unit corresponding to the Serra do Cachimbo and adjacent uplands in northern Mato Grosso and southern Pará.
Within this unit, the high density of rapids, waterfalls, and deeply incised valleys typifies an Extreme Shield setting (Dagosta, de Pinna, 2019), in which geomorphological barriers simultaneously promote allopatric divergence and restrict the establishment of lineages widespread in other Brazilian Shield basins. Therefore, these regions exhibit pronounced faunal regionalization, reduced sympatry, and comparatively low species richness (Dagosta, de Pinna, 2019; Marinho, Dagosta, 2024; Silva et al., 2025). The restricted distribution of M. nanah likely reflects long-term geographic isolation associated with rapids and waterfalls, combined with limited dispersal across drainage divides. Moreover, M. nanah represents the fifth species of this putative group described from the Serra do Cachimbo, all of which are likely endemic to the region. Together with congeners restricted to the Chapada dos Parecis, these species reinforce the recognition of these Amazonian Shield uplands as important regions of endemism for small-bodied freshwater fishes and reinforce the need for continued taxonomic and biogeographic studies in Amazonian Shield headwaters, as previously emphasized by several authors (e.g., Sousa et al., 2010; Lima et al., 2023; Marinho, Dagosta, 2024; Silva et al., 2025).
Comparative material examined. Material examined here is the same listed at Ohara, Marinho (2016), Marinho et al. (2021), and Silva et al. (2025).
Acknowledgments
We thank Osvaldo Oyakawa (MZUSP) and Michel Gianetti (MZUSP) for curatorial assistance, and Angela Zanata (UFBA) for preparing the cleared and stained specimens. We are also grateful to Osvaldo Oyakawa (MZUSP) and Rafael Burger (UFBA) for assistance during fieldwork, Leonardo Oliveira-Silva (UNESP) for photographs of Figs. 1 and 3, and Lívia Fusari (UFSCar) for identifying the insects found in the stomach contents.
References
Costa WJEM. Description of two new species of the genus Moenkhausia (Characiformes: Characidae) from the central Brazil. Zool Anz. 1994; 232(1–2):21–29.
Dagosta FCP, de Pinna M. Biogeography of Amazonian fishes: deconstructing river basins as biogeographic units. Neotrop Ichthyol. 2017; 15(3):e170034. https://doi.org/10.1590/1982-0224-20170034
Dagosta FCP, de Pinna M. The fishes of the Amazon: distribution and biogeographical patterns, with a comprehensive list of species. Bull Am Mus Nat Hist. 2019; 2019(431):1–163. https://doi.org/10.1206/0003-0090.431.1.1
Eigenmann CH. The American Characidae – I. Mem Mus Comp Zool. 1917; 43:1–102.
Ferreira KM, Ribeiro AC, Lima FCT, Silva HP, Ferreira DC, Mirande JM. A new species of Inpaichthys from the rio Canamã, rio Aripuanã basin, Mato Grosso, Brazil, with a redefinition of the genus (Characidae: Stethaprioninae). Neotrop Ichthyol. 2024; 22(1):e230113. https://doi.org/10.1590/1982-0224-2023-0113
Fink WL, Weitzman SH. The so-called Cheirodontin fishes of Central America with description of two new species (Pisces, Characidae). Smithson Contrib Zool. 1974; 172:1–46.
Fricke R, Eschmeyer WN. Eschmeyer’s catalog of fishes: guide to fish collections. [Internet]. San Francisco: California Academy of Sciences; 2026. Available from: https://researcharchive.calacademy.org/research/ichthyology/catalog/collections.Asp
Fricke R, Eschmeyer WN, Van der Laan R. Eschmeyer’s catalog of fishes: genera, species, references [Internet]. San Francisco: California Academy of Sciences; 2026. Available from: http://researcharchive.calacademy.org/research/ichthyology/catalog/fishcatmain.asp
International Union for Conservation of Nature (IUCN). Standards and petitions committee. Guidelines for using the IUCN Red List categories and criteria. Version 15.1 [Internet]. Gland; 2024. Available from: http://cmsdocs.s3.amazonaws.com/RedListGuidelines.pdf
Lima FCT, Britski HA, Machado FA. A new Moenkhausia (Characiformes: Characidae) from central Brazil, with comments on the area relationship between the upper rio Tapajós and upper rio Paraguai systems. Aqua. 2007; 13:45–54.
Lima FCT, Toledo-Piza M. New species of Moenkhausia (Characiformes: Characidae) from the rio Negro of Brazil. Copeia. 2001; 2001(4):1058–63.
Lima AD, Vita G, Dutra GM, Ohara WM, Pastana MNL. A new Moenkhausia (Characiformes: Characidae) from rio Braço Norte, rio Tapajós basin, with comments on the fish endemism of Serra do Cachimbo plateau. Zootaxa. 2023; 5330(4):586–96. https://doi.org/10.11646/zootaxa.5330.4.6
Mariguela TC, Benine RC, Abe KT, Avelino GS, Oliveira C. Molecular phylogeny of Moenkhausia (Characidae) inferred from mitochondrial and nuclear DNA 16 evidence. J Zool Syst Evol Res. 2013; 51(4):327–32. https://doi.org/10.1111/jzs.12025
Marinho MMF, Dagosta FCP. On a new colorful species of Moenkhausia (Characiformes: Characidae) from the upper rio Madeira basin at the Chapada dos Parecis, Brazil, with comments on its conservation and putative biogeographic history. J Fish Biol. 2023; 103(5):1122–28. https://doi.org/10.1111/jfb.15513
Marinho MMF, Dagosta FCP. Redescription of Hyphessobrycon cachimbensis (Characiformes: Characidae) with the description of a new congener from the Serra do Cachimbo, Brazil. Neotrop Ichthyol. 2024; 22(2):e230127. https://doi.org/10.1590/1982-0224-2023-0127
Marinho MMF, Ohara WM, Dagosta FCP. A new species of Moenkhausia (Characiformes: Characidae) from the rio Madeira basin, Brazil, with comments on the evolution and development of the trunk lateral line system in characids. Neotrop Ichthyol. 2021; 19(2):e200118. https://doi.org/10.1590/1982-0224-2020-0118
Marinho MMF, Peixoto L, Loboda T, de Pinna M, Britski H, Menezes NA et al.MZUSP: the ichthyological collection at Museu de Zoologia da Universidade de São Paulo. Bol Soc Bras Ictiol. 2019; 129:95–102.
Melo BF, Ota RP, Benine RC, Carvalho FR, Lima FCT, Mattox GM et al. Phylogenomics of Characidae, a hyper-diverse Neotropical freshwater fish lineage, with a phylogenetic classification including four families (Teleostei: Characiformes). Zool J Linn Soc. 2024; 202(1):zlae101. https://doi.org/10.1093/zoolinnean/zlae101
Mirande JM. Phylogeny of the family Characidae (Teleostei: Characiformes): from characters to taxonomy. Neotrop Ichthyol. 2010; 8(3):385–568. https://doi.org/10.1590/S1679-62252010000300001
Mirande JM. Morphology, molecules and the phylogeny of Characidae (Teleostei, Characiformes). Cladistics. 2019; 35(3):282–300. https://doi.org/10.1111/cla.12345
Ohara WM, Marinho MMF. A new species of Moenkhausia Eigenmann (Characiformes; Characidae) from the upper rio Machado at Chapada dos Parecis, rio Madeira basin, Brazil. Neotrop Ichthyol. 2016; 14(1):e150041.
https://doi.org/10.1590/1982-0224- 20150041
Oliveira C, Avelino GS, Abe KT, Mariguela TC, Benine RC, Ortí G et al.Phylogenetic relationships within the speciose family Characidae (Teleostei: Ostariophysi: Characiformes) based on multilocus analysis and extensive ingroup sampling. BMC Evol Biol. 2011; 11:275. https://doi.org/10.1186/1471-2148-11-275
Reia, L, Silva GSC, Oliveira C, Benine RC. New reddish species of Moenkhausia Eigenmann (Characiformes: Characidae) from the upper rio Xingu basin, Brazil. Neotrop Ichthyol. 2024; 22(1):e230089. https://doi.org/10.1590/1982-0224-2023-0089
Silva JI, Santana Y, Marinho MMF. New species of Moenkhausia (Characiformes: Acestrorhamphidae) from the Amazon basin at Serra do Cachimbo, Pará, Brazil. Neotrop Ichthyol. 2025; 23(3):e250089. https://doi.org/10.1590/1982-0224-2025-0089
Sousa LM, Netto-Ferreira AL, Birindelli JLO. Two new species of Moenkhausia Eigenmann (Characiformes: Characidae) from Serra do Cachimbo, Pará, Northern Brazil. Neotrop Ichthyol. 2010; 8(2):255–64. http://dx.doi.org/10.1590/S1679-62252010000200003
Taylor WR, Van Dyke GC. Revised procedures for staining and clearing small fishes and other vertebrates for bone and cartilage study. Cybium. 1985; 9(2):107–19.
Authors

Priscila Camelier1 and Manoela Maria Ferreira Marinho2
[1] Programa de Pós-Graduação em Biodiversidade e Evolução, Instituto de Biologia, Universidade Federal da Bahia, Rua Barão de Jeremoabo, 147, Ondina, 40170-115, Salvador, BA, Brazil. pricamelier@gmail.com (corresponding author).
[2] Laboratório de Zoologia, Instituto de Biociências, Universidade Federal de Mato Grosso do Sul, Bairro Universitário, 79070-900, Campo Grande, MS, Brazil. manoela.marinho@ufms.br.
Authors’ Contribution 

Priscila Camelier: Conceptualization, Data curation, Formal analysis, Funding acquisition, Investigation, Methodology, Visualization, Writing-original draft, Writing-review and editing.
Manoela Maria Ferreira Marinho: Conceptualization, Data curation, Formal analysis, Funding acquisition, Investigation, Methodology, Visualization, Writing-original draft, Writing-review and editing.
Ethical Statement
Collection permit number SISBio 21924-1.
Competing Interests
The author declares no competing interests.
Data availability statement
The authors confirm that the data supporting the findings of this study are available within the article.
AI statement
The authors did not use any AI-assisted technologies in the creation of this manuscript or its figures.
Funding
The authors were funded by Conselho Nacional de Desenvolvimento Científico e Tecnológico – CNPq (MMFM and PC, grant #405706/2022–7; PC, grants #423760/2018–1 and #404826/2023–7; MMFM grant #401422/2025–9); Fundação de Amparo à Pesquisa do Estado da Bahia – FAPESB (PC, grant #APP0037–2023); Fundação de Amparo à Pesquisa do Estado de São Paulo – FAPESP (South American Characiformes Inventory Project, grant #2011/50282–7); Universidade Federal da Paraíba – UFPB (MMFM, grant #PROPESQ/PRPG PIA 13512–2020).
Peer Review
How to cite this article
Camelier P, Marinho MMF. Description of a new species of Moenkhausia (Characiformes: Acestrorhamphidae) from tributaries of rio Tapajós basin at Serra do Cachimbo, Pará State, Brazil. Neotrop Ichthyol. 2026; 24(3):e260067. https://doi.org/10.1590/1982-0224-2026-0067
Copyright
This is an open access article under the terms of the Creative Commons Attribution License, which permits use, distribution and reproduction in any medium, provided the original work is properly cited.
Distributed under
Creative Commons CC-BY 4.0

© 2025 The Authors.
Diversity and Distributions Published by SBI
 Accepted August 3, 2026
Submitted April 23, 2026
Epub October 20, 2026